Ocean Carbon & Biogeochemistry
Studying marine ecosystems and biogeochemical cycles in the face of environmental change
  • Home
  • About OCB
    • About Us
    • Scientific Breadth
      • Biological Pump
      • Changing Marine Ecosystems
      • Changing Ocean Chemistry
      • Estuarine and Coastal Carbon Fluxes
      • Ocean Carbon Uptake and Storage
      • Ocean Observatories
    • Code of Conduct
    • Get Involved
    • Project Office
    • Scientific Steering Committee
    • OCB committees
      • OCSIF – Ocean Carbonate System Intercomparison
      • Ocean-Atmosphere Interaction
      • Ocean Time-series
      • US Biogeochemical-Argo
  • Activities
    • 20 years of OCB Symposium – 18 November 2026
    • OCB Webinars
    • Summer Workshop
    • Guidelines for OCB Workshops & Activities
    • Topical Workshops
      • 7th DMS(P) Symposium
      • Marine Virus Workshop
      • Completed
        • CMIP6 Models Workshop
        • Coastal BGS Obs with Fisheries
        • C-saw extreme events workshop
        • Expansion of BGC-Argo and Profiling Floats
        • Fish, fisheries and carbon
        • Future BioGeoSCAPES program
        • GO-BCG Scoping Workshop
        • Lateral Carbon Flux in Tidal Wetlands
        • Leaky Deltas Workshop
        • Marine CDR Workshop
        • Ocean Nucleic Acids ‘Omics
        • Pathways Connecting Climate Changes to the Deep Ocean
    • Small Group Activities
      • BECS Benthic Ecosystem and Carbon Synthesis WG
      • Metabarcoding intercal WG
      • Meta-eukomics WG
      • Metaproteomic Intercomparison
      • SedMIP
      • Recently completed
        • Aquatic Continuum OCB-NACP Focus Group
        • Arctic-COLORS Data Synthesis
        • Carbon Isotopes in the Ocean Workshop
        • CMIP6 WG
        • Filling the gaps air–sea carbon fluxes WG
        • Fish Carbon WG
        • mCDR
        • Mixotrophs & Mixotrophy WG
        • N-Fixation WG
        • Ocean Carbonate System Intercomparison Forum
        • Ocean Carbon Uptake WG
        • OOI BGC sensor WG
        • Operational Phytoplankton Observations WG
        • Phytoplankton Taxonomy WG
    • Other Workshops
    • Science Planning
      • Coastal CARbon Synthesis (CCARS)
      • North Atlantic-Arctic
    • Ocean Acidification PI Meetings
    • Training Activities
      • PACE Hackweek 2025
      • PACE Hackweek 2024
      • PACE Training Activity 2022
  • Science Support
    • OCB Activity Proposal Solicitation
    • Guidelines for OCB Workshops & Activities
    • Data management and archival
    • Early Career
    • Funding Sources
    • Jobs & Postdocs
    • Meeting List
    • OCB Topical Websites
      • Ocean Fertilization
      • Trace gases
      • US IIOE-2
    • Outreach & Education
    • Promoting your science
    • Student Opportunities
    • Travel Support
  • Publications
    • OCB Workshop Reports
    • Science Planning and Policy
    • Newsletter Archive
  • Science Highlights
  • News

Archive for New OCB Research – Page 6

Turbulent Mixing: A Dominant Source of Oxygen in the Upper Equatorial Pacific

Posted by mmaheigan 
· Tuesday, March 12th, 2024 

What balances oxygen removal in the equatorial Pacific? For a long time, oxygen in the eastern and central tropical Pacific was assumed to be mainly supplied by the large-scale advection of remotely ventilated waters via the equatorial current system and meridional circulation. A recent study used an eddy-resolving simulation of a global ocean model to show that turbulent mixing and its regulation by mesoscale eddies play a critical role in balancing oxygen removal (by consumption and upwelling) in the upper thermocline. Deeper in the water column, mean advection by the zonal currents and meridional circulation dominates. This mixing is tightly regulated by tropical instability waves, which intensify the shear between the equatorial currents and enhance the downward turbulent mixing flux of oxygen into the thermocline. Mesoscale phenomena thus play an indirect yet critical role as a local pathway of ventilation in this region. Testing these model-based hypotheses in the real ocean through dedicated field studies and long-term observations is needed to advance our understanding of the observed expansion of the oxygen deficient zones (ODZs) and model their future trajectory in a warmer and more stratified ocean.
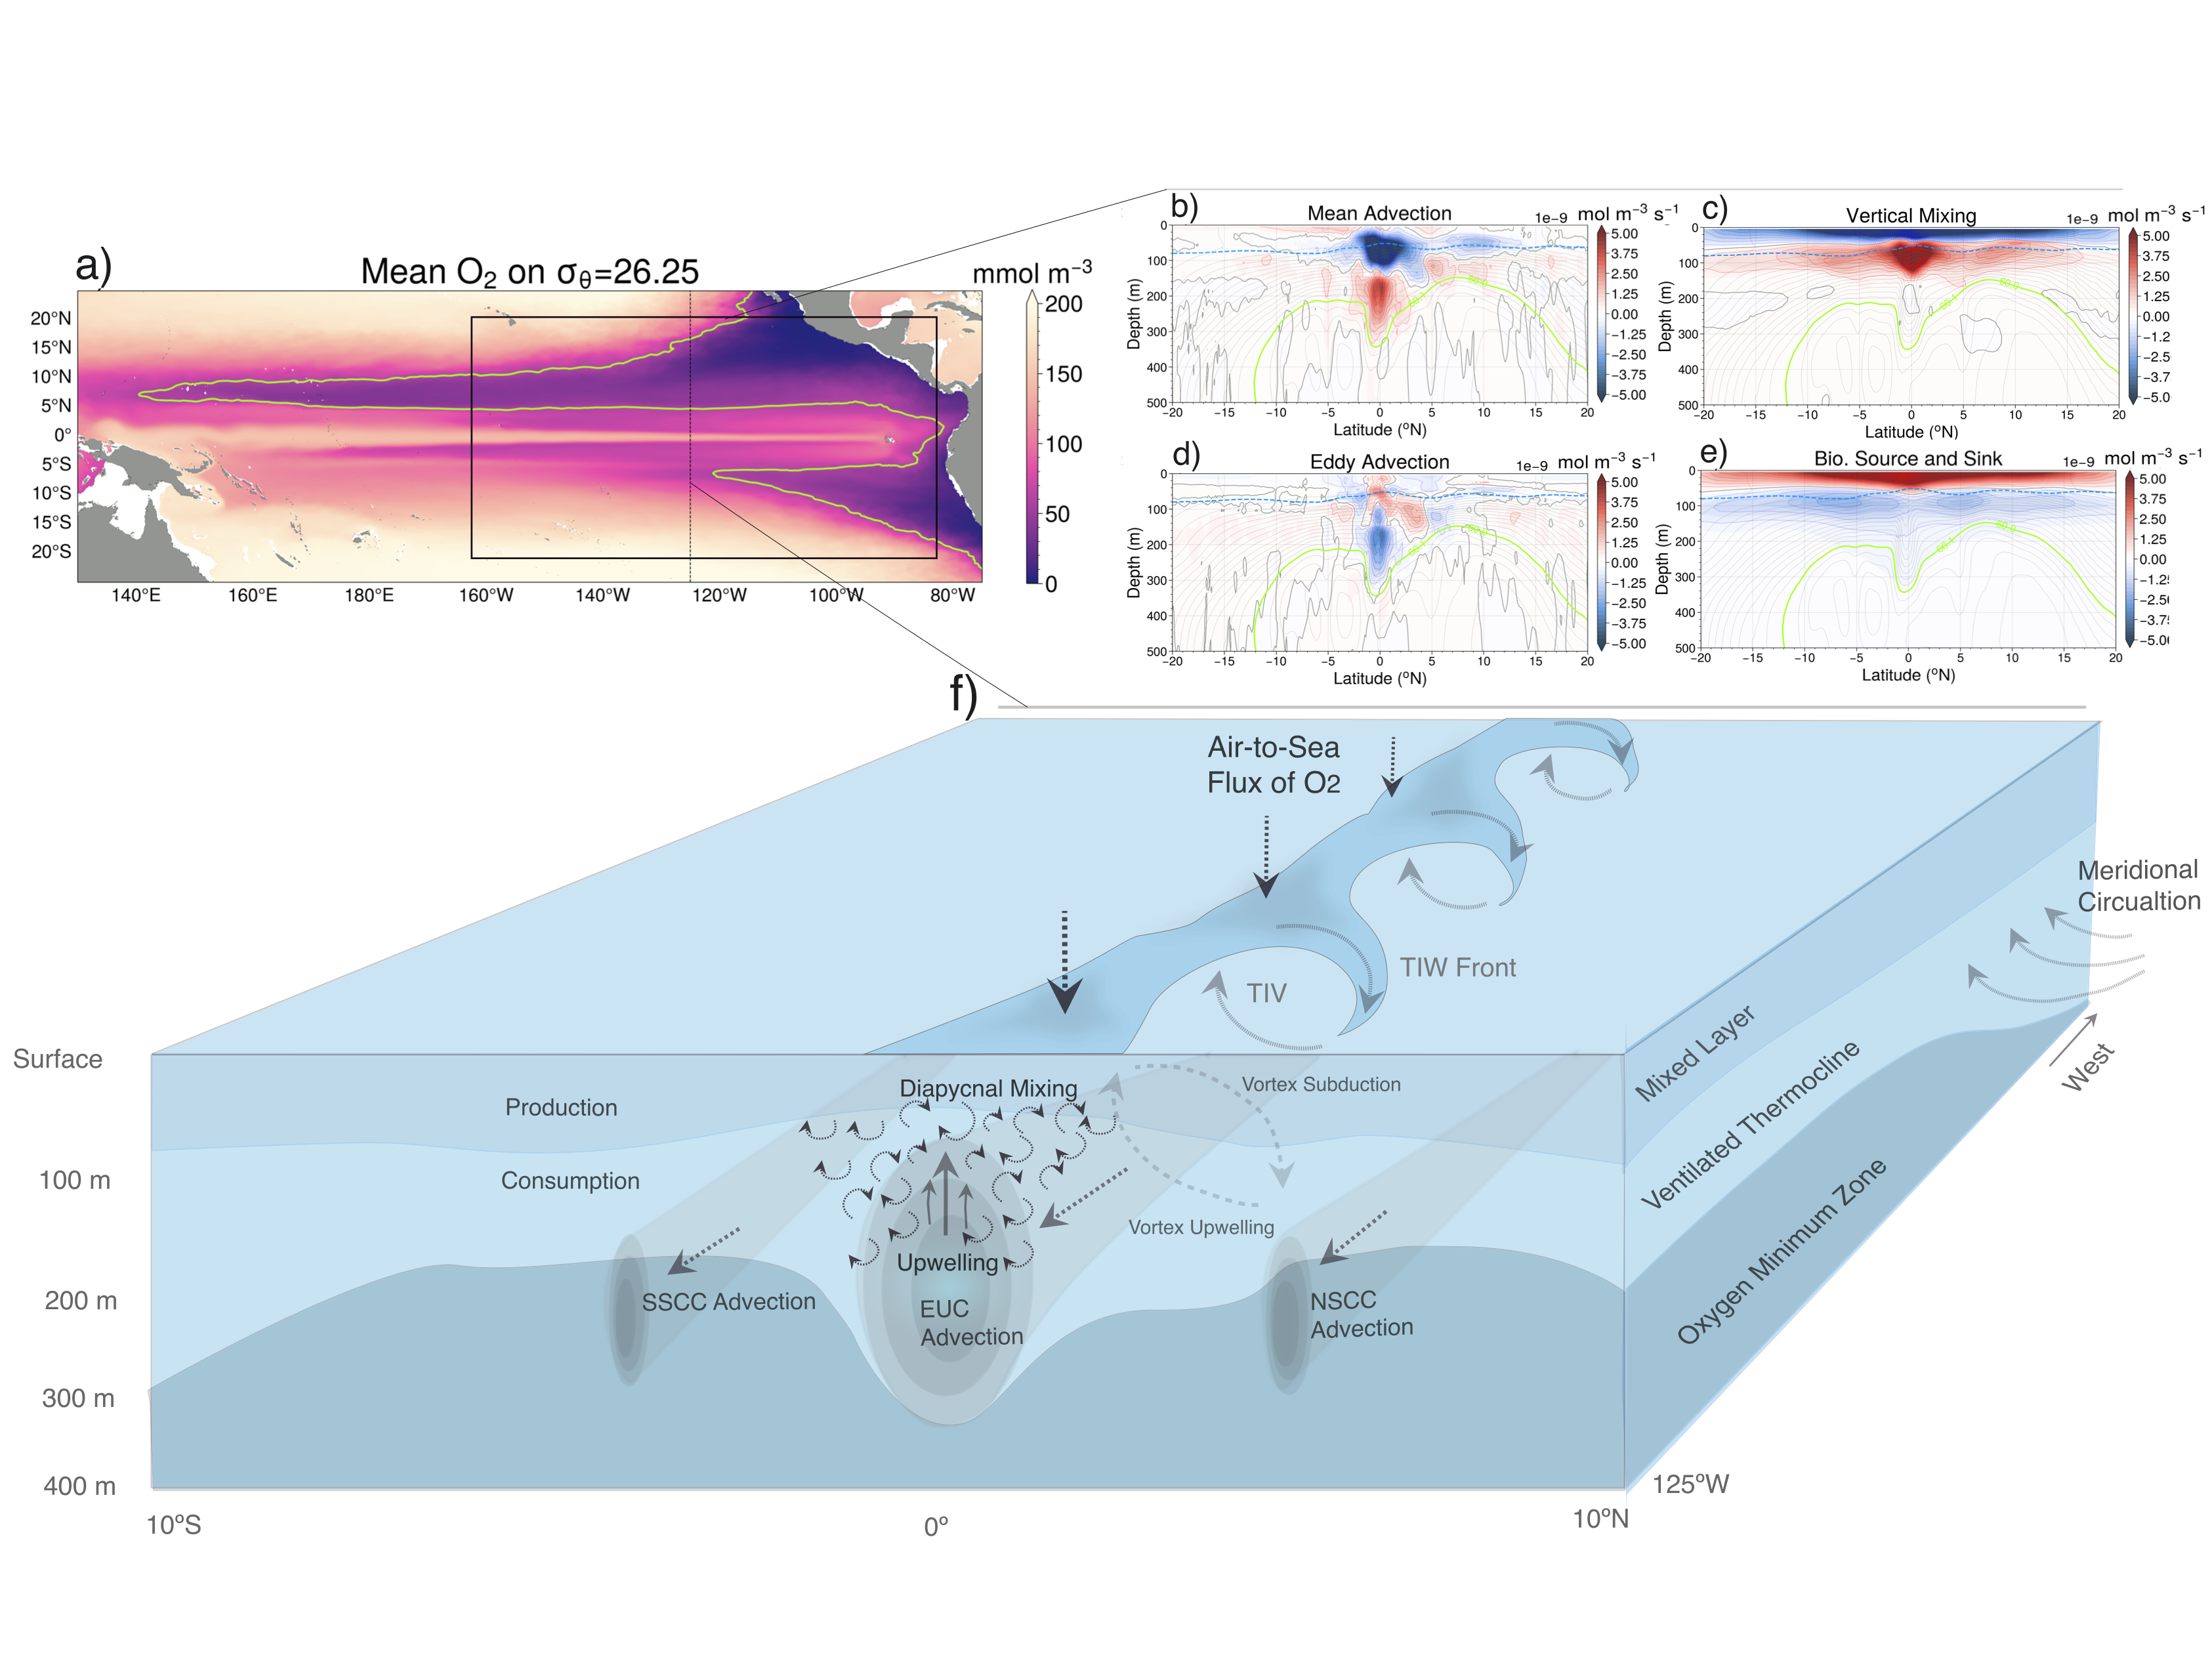
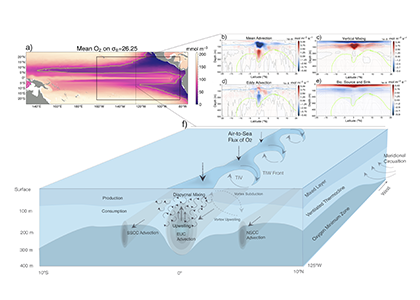
Figure: The main processes that set the mean structure of oxygen in the equatorial Pacific are assessed in an eddy resolving simulation of the Community Earth System Model (CESM). Panel a shows the climatological oxygen distribution on the 26.25 isopycnal in CESM. Panels b-e show the contribution of advection by mean circulation and eddies, vertical mixing, and production and consumption. These processes are illustrated in panel f). Figure adapted from Eddebbar et al (2024).

Authors
Yassir A. Eddebbar (Scripps Institution of Oceanography)
Daniel B. Whitt (NASA Ames)
Ariane Verdy, (Scripps Institution of Oceanography)
Matthew R. Mazloff (Scripps Institution of Oceanography)
Aneesh C. Subramanian (CU Boulder)
Matthew C. Long, (National Center for Atmospheric Research)
Tiny parasites, big impact: Species networks and carbon recycling in an oligotrophic ocean

Posted by mmaheigan 
· Tuesday, March 12th, 2024 

Parasites are everywhere in the ocean. Including the microbial realm where a diverse, widespread group of protist parasites (Syndiniales) infect and kill a range of hosts, such as dinoflagellates, radiolarians, and even larger zooplankton. A complete Syndiniales infection cycle is only 2-3 days. First, the parasite is a free-living spore. Once inside a host, the parasite consumes the host’s carbon and becomes a larger multicellular organism (a trophont) eventually causing the host to burst open and release hundreds of new spores.

Like viruses, parasite lysis is expected to reroute organic carbon to the microbial loop, potentially decreasing the amount of carbon available for export to the deep sea. Yet, the role of Syndiniales in carbon cycling has been hard to define, as depth-specific infection dynamics and links to carbon export remain poorly understood.

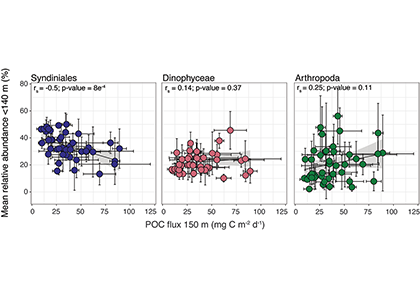
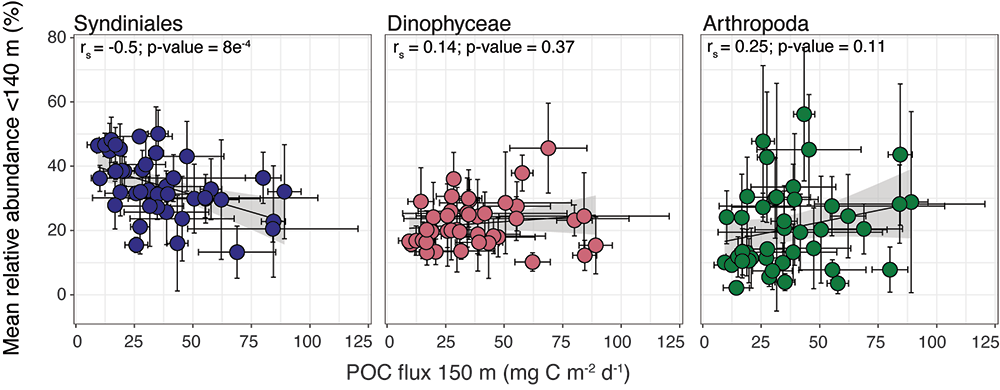
Figure 1. The mean relative abundance of Syndiniales (purple) in the photic zone (<140 m) is negatively correlated with particulate organic carbon (POC) flux at 150 m (p-value < 0.001). Similar correlations are not significant (p-values > 0.05) for other major 18S taxonomic groups, like Dinophyceae (red) and Arthropoda (green).

In a recent study published in ISME Communications, authors analyzed an 18S rRNA gene metabarcoding dataset from the Bermuda Atlantic Time-series Study (BATS) site that included 4 years (2016-2019) and twelve depths (1-1000 m). Syndiniales were the most dominant 18S group at BATS, present throughout the photic and aphotic zones. These parasites were prominent in species networks constructed with 18S sequence data, with significant associations with dinoflagellates and copepods in the surface, and with radiolarians in the aphotic zone. In addition, Syndiniales were the only major 18S group to be significantly (and negatively) correlated to particulate carbon flux (at 150 m), which was estimated from sediment trap data collected concurrently at BATS (Figure 1). This is in situ evidence of flux attenuation among Syndiniales, as they recycle host carbon that would otherwise transfer up to larger organisms (e.g., via grazing). Lastly, authors found 19% of the Syndiniales community is linked between photic and aphotic zones, indicating that parasites are sinking on particles and/or are recirculated via diel vertical migration. Overall, these findings elevate the role of Syndiniales in microbial food webs and further emphasize the importance in quantifying parasite-host dynamics to inform ocean carbon models.


Authors
Sean Anderson (University of New Hampshire / Woods Hole Oceanographic Institution)
Leocadio Blanco-Bercial (Bermuda Institute of Ocean Sciences / Arizona State University)
Craig Carlson (University of California, Santa Barbara)
Elizabeth Harvey (University of New Hampshire)

Coastal DOM database – CoastDOM v1

Posted by hbenway 
· Wednesday, February 28th, 2024 

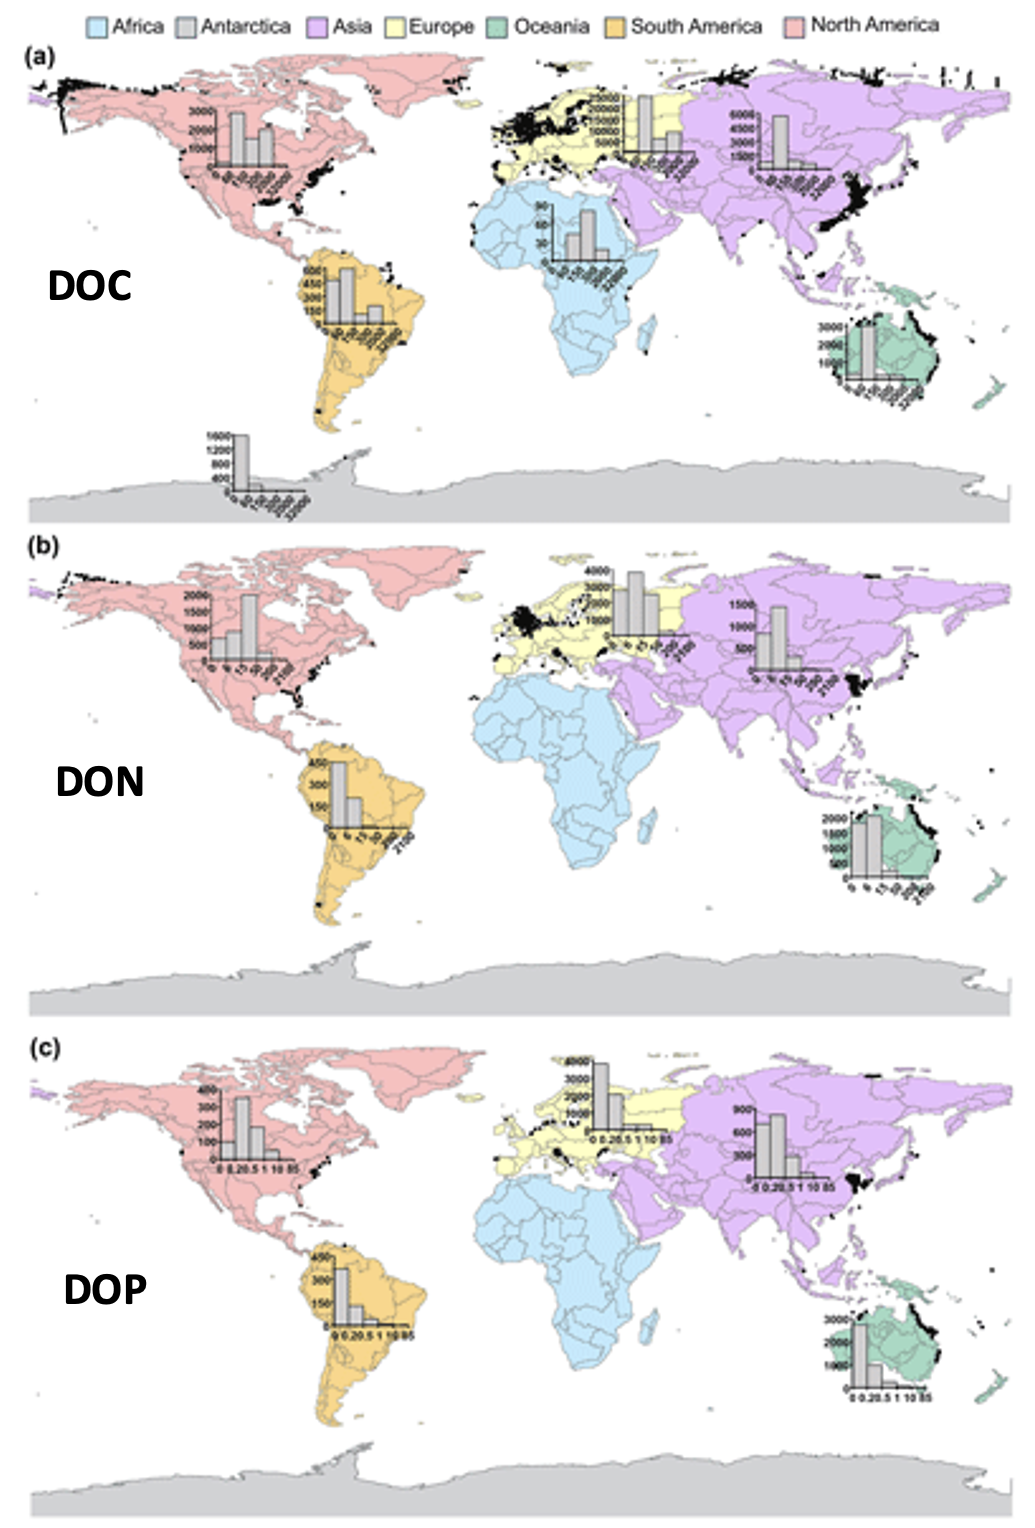
We present the first edition of a global database (CoastDOM v1) and a resulting data manuscript, which compiles previously published and unpublished measurements of DOC, DON, and DOP in coastal waters, consisting of 62,338 (DOC), 20,356 (DON), and 13,533 (DOP) data points, respectively.

CoastDOM v1 includes observations of concentrations from all continents between 1978 and 2022. However, most data were collected in the Northern Hemisphere, with a clear gap in DOM measurements from the Southern Hemisphere.

This dataset will be useful for identifying global spatial and temporal patterns in DOM and will help facilitate the reuse of DOC, DON, and DOP data in studies aimed at better characterizing local biogeochemical processes; closing nutrient budgets; estimating carbon, nitrogen, and phosphorous pools; and establishing a baseline for modelling future changes in coastal waters.

The aim is to publish an updated version of the database periodically to determine global trends of DOM levels in coastal waters, and so if you have DOM data lying around, please submit it to Christian Lønborg (c.lonborg@ecos.au.dk).

CITATIONS

Lønborg et al. 2024. A global database of dissolved organic matter (DOM) concentration measurements in coastal waters (CoastDOM v1), Earth Syst. Sci. Data, 16, 1107–1119, https://doi.org/10.5194/essd-16-1107-2024

Lønborg et al. 2023.A global database of dissolved organic matter (DOM) concentration measurements in coastal waters (CoastDOM v.1). PANGAEA, https://doi.org/10.1594/PANGAEA.964012

Two OCB-led articles featured in AGU Eos Feb. Oceans Issue

Posted by hbenway 
· Friday, January 26th, 2024 

A Closer Look-Sea at the Ocean’s Carbon Cycle

AGU Eos highlights the following two articles emerging from OCB-led activities, including the OCB 2022 plenary session on the biological carbon pump and the 2022 OCB Workshop Marine Carbon Dioxide Removal: Essential Science and Problem Solving for Measurement, Reporting, and Verification.

  • Our Evolving Understanding of Biological Carbon Export
  • The Science We Need to Assess Marine Carbon Dioxide Removal

New synthesis of global ocean greenhouse gas fluxes

Posted by hbenway 
· Friday, January 26th, 2024 

Resplandy, L., Hogikyan, A., Müller, J. D., Najjar, R. G., Bange, H. W., Bianchi, D., et al. (2024). A synthesis of global coastal ocean greenhouse gas fluxes. Global Biogeochemical Cycles, 38, e2023GB007803. https://doi.org/10.1029/2023GB007803.

New framework reveals gaps in US ocean biodiversity protection

Posted by hbenway 
· Friday, January 26th, 2024 

Gignoux-Wolfsohn et al., New framework reveals gaps in US ocean biodiversity protection, OneEarth (2023), https:// doi.org/10.1016/j.oneear.2023.12.014. (accompanying fact sheet)

Ocean iron fertilization may amplify pressures on marine biomass with only a limited climate benefit

Posted by hbenway 
· Friday, January 26th, 2024 

Amidst a heightened focus on the need for both drastic and immediate emissions reductions and carbon dioxide removal to limit warming to 1.5°C (IPCC, 2022), attention is returning to ocean iron fertilization (OIF) as a means of marine carbon dioxide removal (mCDR). First discussed in the early 1990s by John Martin, the concept posits that fertilization of iron-limited marine phytoplankton would lead to enhanced ocean carbon storage via a stimulation of the ocean’s biological carbon pump. However, we lack knowledge about how OIF might operate in concert with an ocean responding to climate change and what the consequences of altered nutrient consumption patterns might be for marine ecosystems, particularly for fisheries in national exclusive economic zones (EEZs). Tagliabue et al. (2023) addressed this in a recent study using state-of-the-art climate, ocean biogeochemical, and ecosystem models under a high-emissions scenario.

The study’s findings suggested that  OIF can contribute at most a few 10s of Pg of mCDR under a high-emissions climate change scenario. This is equivalent to fewer than five years of current emissions and is consistent with earlier modeling assessments. This estimate is based on the modeled representation of carbon and iron cycling and a highly efficient OIF strategy that may be difficult to achieve in practice. Enhanced surface uptake of major nutrients due to OIF also led to a drop in global net primary production, in addition to that due to climate change alone. By then coupling a complex model of upper trophic levels, the projected declines in animal biomass due to climate change were amplified by around a third due to OIF, with the most negative impacts projected to occur in the low latitude EEZs, which are already facing increasing pressures due to climate change.

This work highlights feedbacks within the ocean’s biogeochemical and ecological systems in response to OIF that emerged over large spatial and temporal scales. Associated pressures on marine ecosystems pose major challenges for proposed management and monitoring. Restricting OIF to the highest latitudes of the Southern Ocean might mitigate some of these negative effects, but this only further reduces the minor mCDR benefit, suggesting that OIF may not make a significant contribution.

Authors
A. Tagliabue (Univ. Liverpool)
B. S. Twining (Bigelow Laboratory)
N. Barrier & O. Maury (MARBEC, IRD, IFREMER, CNRS, Université de Montpellier, France)
M. Berger & Laurent Bopp (ENS-LMD, Paris, France)

IPCC. Summary for Policymakers. in Climate Change, 2022: Mitigation of Climate Change. Contribution of Working Group III to the Sixth Assessment Report of the Intergovernmental Panel on Climate Change (eds. Shukla, P. R. et al.) (Cambridge University Press, 2022).

Addressing the problem of additionality in ocean alkalinity enhancement

Posted by hbenway 
· Friday, January 26th, 2024 

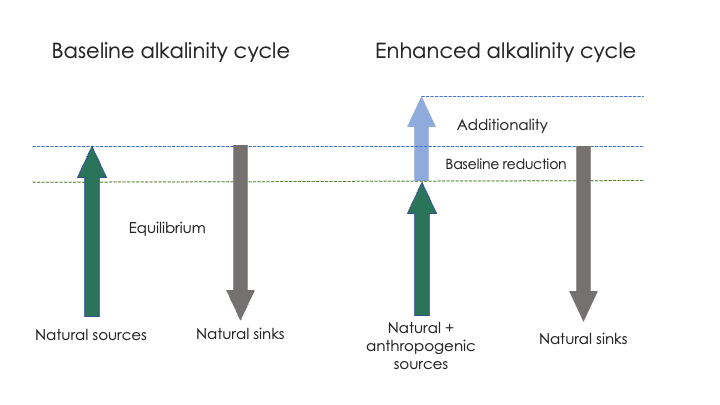
The ultimate goal of marine carbon dioxide (CO2) removal (mCDR) is to sequester more atmospheric CO2 in the ocean than the ocean already does today. As such, any mCDR deployment must lead to quantifiably more CO2 sequestration in the ocean than would have happened without the deployment. This requirement is referred to as “additionality.”

To understand how additionality of CO2 removal is relevant for Ocean Alkalinity Enhancement (OAE) we need to recall what OAE seeks to do. Essentially, OAE accelerates a natural process (weathering) that absorbs protons (H+) in liquid media through geochemical reactions. This anthropogenically enhanced “buffering” results in fewer freely available protons and thus a shift in the marine carbonate system away from CO2 and towards carbonate ions (CO32+), a shift that enables oceanic uptake of atmospheric CO2. However, the anthropogenically buffered protons are then no longer available to be absorbed by natural weathering processes (e.g., calcium carbonate dissolution). Therefore, anthropogenic buffering of seawater pH partially replaces natural buffering (and associated CO2 sequestration) that would have occurred in the absence of OAE. A recent paper (Bach, 2024) describes this “additionality problem” in the context of OAE, and through a series of incubation experiments that emulate a high-energy wave zone (constant mixing), the author investigates how different forms of anthropogenic alkalinity (e.g., sodium hydroxide, steel slag, and olivine) interact with natural alkalinity sources (beach sand) and the subsequent impacts on atmospheric CO2 drawdown. While many questions will require more targeted study, this study represents a foundational baseline for future OAE experimentation and provides preliminary insights on siting and methods of anthropogenic alkalinity addition.

Figure caption: Simple schematic of the additionality problem. In the baseline state (left), alkalinity sources and sinks are (assumed to be) in equilibrium. The addition of an anthropogenic alkalinity source (right) to the baseline system may reduce alkalinity inputs via natural sources. The reduction of natural sources must be subtracted from the anthropogenic sources to correctly calculate the additional CO2 sequestration potential of OAE.

Author
Lennart Bach (Univ. Tasmania)

New paper published by OCB Ocean Carbonate System Intercomparison Forum (OCSIF)

Posted by hbenway 
· Wednesday, January 3rd, 2024 

Carter, B.R., Sharp, J.D., Dickson, A.G., Álvarez, M., Fong, M.B., García-Ibáñez, M.I., Woosley, R.J., Takeshita, Y., Barbero, L., Byrne, R.H., Cai, W.-J., Chierici, M., Clegg, S.L., Easley, R.A., Fassbender, A.J., Fleger, K.L., Li, X., Martín-Mayor, M., Schockman, K.M. and Wang, Z.A. (2023), Uncertainty sources for measurable ocean carbonate chemistry variables. Limnol Oceanogr. https://doi.org/10.1002/lno.12477

Learn more about OCSIF here.

Fishing Vessel Ocean Observing Network (FVON) reimagines the global data collection paradigm

Posted by mmaheigan 
· Friday, December 1st, 2023 

With an increasingly wide variety of technology and innovations, from buoys to satellites, we now understand the open ocea n better than ever. Yet, existing technologies cannot cost-effectively provide accurate, up-to-date data on coastal and shelf ocean environments, especially beneath the surface. These dynamic regions impact billions of people in profound and varied ways.

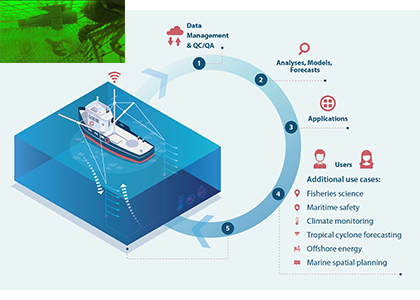
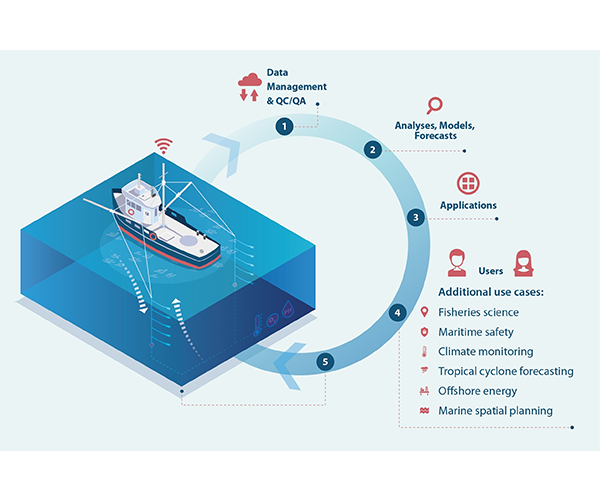
Figure caption: Alongside other major global ocean observing technologies and networks, the Fishing Vessel Ocean Observing Network is built around the concept of “fishing for data” to collect high-quality ocean data such as temperature and salinity profiles. These measurements inform critical policy decisions, are integrated into sustainability efforts for fishers, scientists, and other relevant stakeholders, and can improve climate resiliency while protecting the health, well-being, and livelihoods of coastal communities and participants in the blue economy.

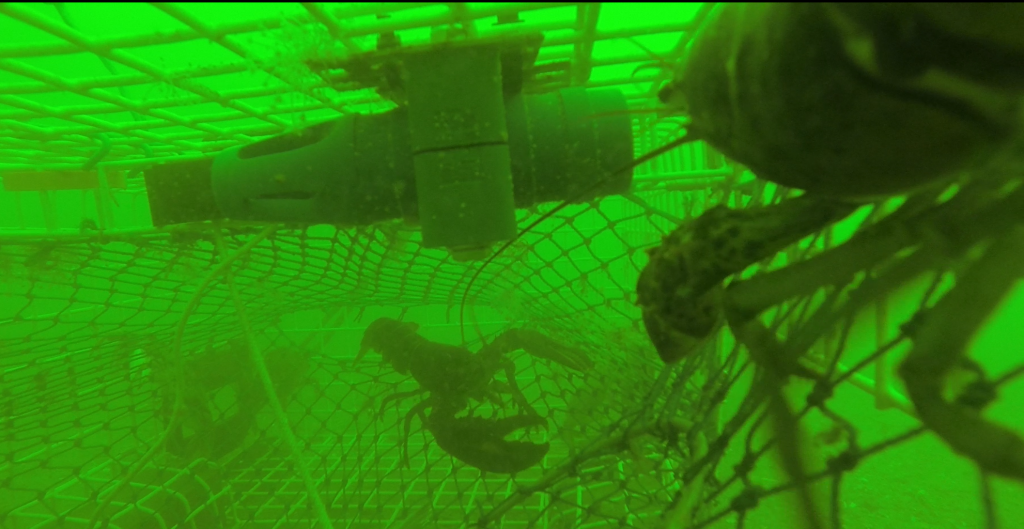
As described in a recent publication, the Fishing Vessel Ocean Observing Network (FVON) is reimagining the global data collection paradigm of coastal and shelf oceans by partnering with fishers and regional observation networks around the world. With more than four million fishing vessels worldwide, fishers cover much of the data-sparse nearshore ocean environments, vitally important regions of the ocean. By outfitting sensors onto vessels and on fishing gear, programs from New Zealand to Japan to New England, including researchers at WHOI, demonstrate that fishers can participate actively in the ongoing data revolution and eliminate critical oceanic data gaps without changing their standard fishing activities. Exponentially increasing the scale of data collection through fishing vessel and gear-based observations in nearshore marine environments has and will continue to democratize ocean observation, improve weather forecasting and ocean monitoring, and promote sustainable fishing while safeguarding lives and livelihoods. Already a proven concept regionally, FVON, alongside fishers and regional observation networks, will expand fishing-based observation to a global initiative.


Authors
Cooper Van Vranken (Ocean Data Network)
Julie Jakoboski (MetOcean Solutions, New Zealand)
John W. Carroll (Ocean Data Network)
Christopher Cusack (Environmental Defense Fund)
Patrick Gorringe (Swedish Meteorological and Hydrological Institute)
Naoki Hirose (Kyushu University, Japan)
James Manning (NOAA Northeast Fisheries Science Center (retired))
Michela Martinelli (National Research Council−Institute of Marine Biological Resources and Biotechnologies, Italy)
Pierluigi Penna (National Research Council−Institute of Marine Biological Resources and Biotechnologies, Italy)
Mathew Pickering (Environmental Defense Fund)
A. Miguel Piecho-Santos (Portuguese Institute for Sea and Atmosphere)
Moninya Roughan (University of New South Wales, Australia)
João de Souza (MetOcean Solutions, New Zealand)
Hassan Moustahfid (NOAA Integrated Ocean Observing System (IOOS))

« Previous Page
Next Page »

FilterbyKeyword

abundance acidification additionality advection africa aggregates air-sea air-sea interactions albedo algae alkalinity allometry amendments ammonium AMO AMOC anoxic Antarctic Antarctica anthro impacts anthropogenic carbon anthropogenic impacts appendicularia aquaculture aquatic continuum aragonite saturation arctic Argo argon arsenic artificial seawater assumptions AT Atlantic atmosphere atmospheric CO2 atmospheric nitrogen deposition authigenic carbonates autonomous platforms AUVs awb bacteria bathypelagic BATS BCG Argo benthic bgc argo bias bio-go-ship bio-optical bioavailability biogeochemical biogeochemical cycles biogeochemical models biogeochemistry Biological Essential Ocean Variables biological pump biomass biophysics bloom blue carbon bottom water boundary layer buffer capacity C14 CaCO3 calcification calcite carbon carbon-climate feedback carbon-sulfur coupling carbon 14 carbonate carbonate chemistry carbonate chemistry OAE carbonate system carbon budget carbon cycle carbon cycling carbon dioxide carbon export carbon fluxes carbon removal carbon sequestration carbon storage Caribbean CCA CCS CDOM changing marine chemistry changing marine ecosystems changing marine environments changing ocean chemistry chemical oceanographic data chemical speciation chemoautotroph chesapeake bay chl a chlorophyll circulation climate clouds CO2 CO3 coastal and estuarine coastal darkening coastal ocean cobalt Coccolithophores commercial community community composition competition conservation cooling effect copepod copepods coral reefs cruise CTD currents cyclone daily cycles data data access data assimilation database data management data product data sets Data standards DCM dead zone decadal trends decomposers decomposition deep convection deep ocean deep sea coral deep water deepwater horizon denitrification dense water deoxygenation depth diatoms DIC diel migration diffusion dimethylsulfide dinoflagellate dinoflagellates discrete measurements disequilibrium distribution DOC DOM domoic acid DOP dust DVM earth system ecological feedbacks ecology economics ecosystem management ecosystems eddy Education EEZ Ekman transport emissions ENSO enzyme equatorial current equatorial regions ESM estuarine and coastal carbon fluxes estuary euphotic zone eutrophication evolution export export fluxes export production extreme events faecal pellets fecal pellets feces feeding filter feeders filtration rates fire fish Fish carbon fisheries fishing fjord float floats fluid dynamics fluorescence food webs forage fish forams framework freshening freshwater frontal zone fronts functional role fungi future oceans gelatinous zooplankton gene transfer geochemistry geoengineering geologic time GEOTRACES glaciers gliders global carbon budget global oceam global ocean global ocean models global overturning circulation global warming go-ship gradient grazing greenhouse gas greenhouse gases Greenland ground truthing groundwater Gulf of Maine Gulf of Mexico Gulf Stream gyre harmful algal bloom heat waves high latitude human food human impact human well-being hurricane hydrogen hydrothermal hypoxia ice age iceberg ice cores ice cover industrial onset inland waters in situ inverse circulation ions iron iron fertilization iron limitation isotopes jellies katabatic winds kelvin waves krill kuroshio lab vs field lagoon land land-ocean continuum larvaceans lateral transport LGM lidar ligands light light attenuation lineage lipids low nutrient machine learning mangroves marine carbon cycle marine heatwave marine particles marine snow marine snowfall marshes mCDR mechanisms Mediterranean meltwater mesocosm mesopelagic mesoscale mesoscale processes metagenome metals methane methods microbes microbial processes microlayer microorganisms microplankton microplastics microscale microzooplankton midwater migration minerals mitigation mixed layer mixed layers mixing mixotrophs mixotrophy model modeling modeling atmosphere model validation mode water molecular diffusion MPT MRV multi-decade N2 n2o NAAMES NCP nearshore net community production net primary productivity new ocean state new technology Niskin bottle nitrate nitrogen nitrogen cycle nitrogen fixation nitrous oxide north atlantic north pacific North Sea NPP nuclear war nutricline nutrient budget nutrient cycles nutrient cycling nutrient limitation nutrients OA observations ocean-atmosphere ocean acidification ocean acidification data ocean alkalinity enhancement ocean carbon uptake & storage ocean carbon uptake and storage ocean color ocean interior ocean modeling ocean observatories ocean warming ODZ oil oligotrophic omics OMZ open ocean optics organic carbon organic particles oscillation outwelling overturning circulation oxidizing oxygen oxygen-deficient pacific paleoceanography PAR parameter optimization parasite particle flux particles partnerships pathway pCO2 PDO peat pelagic perturbation PETM pH phenology phosphate phosphorus photosynthesis physical processes physiology phytoplankton PIC piezophilic piezotolerant plankton POC polar polar regions policy pollutants precipitation predation predator-prey predators prediction pressure primary productivity Prochlorococcus productivity prokaryotes proteins pteropods pycnocline python radioisotopes rain redox remineralization remote sensing repeat hydrography residence time resource management respiration resuspension rivers rocky shore Rossby waves Ross Sea ROV salinity salt marsh satellite scale seafloor seagrass sea ice sea level rise seasonal seasonal effects seasonality seasonal patterns seasonal trends sea spray sea surface seawater collection seaweed secchi sediments sensor sensors sequestration shelf ocean shelf system shells ship-based obs ship-based observations shorelines siderophore silica silicate silicon cycle sink sinking sinking particles size SOCCOM soil carbon solubility pump southern ocean south pacific spatial covariations speciation spring mixing SST state estimation stoichiometry stratification subduction submesoscale subpolar subtropical sulfate surf surface surface ocean surface water surface waters Synechococcus technology teleconnections temperate temperature temporal covariations thermocline thermodynamics thermohaline thorium tidal time time-series time of emergence titration top predators total alkalinity trace elements trace metals trait-based transfer efficiency transient features trawling Tris trophic interactions trophic transfer tropical turbulence twilight zone upper ocean upper water column upwelling US CLIVAR uvp validation velocity gradient ventilation vertical flux vertical migration vertical transport viruses warming water clarity water column water mass water quality waves weathering western boundary currents wetlands winter mixing zooplankton

Copyright © 2026 - OCB Project Office, Woods Hole Oceanographic Institution, 266 Woods Hole Rd, MS #25, Woods Hole, MA 02543 USA Phone: 508-289-2838  •  Fax: 508-457-2193  •  Email: ocb_news@us-ocb.org

link to nsflink to noaalink to WHOI

Funding for the Ocean Carbon & Biogeochemistry Project Office is provided by the National Science Foundation (NSF) and the National Aeronautics and Space Administration (NASA). The OCB Project Office is housed at the Woods Hole Oceanographic Institution.