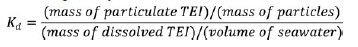
Ocean Carbon & Biogeochemistry
Studying marine ecosystems and biogeochemical cycles in the face of environmental change
  • Home
  • About OCB
    • About Us
    • Scientific Breadth
      • Biological Pump
      • Changing Marine Ecosystems
      • Changing Ocean Chemistry
      • Estuarine and Coastal Carbon Fluxes
      • Ocean Carbon Uptake and Storage
      • Ocean Observatories
    • Code of Conduct
    • Get Involved
    • Project Office
    • Scientific Steering Committee
    • OCB committees
      • OCSIF – Ocean Carbonate System Intercomparison
      • Ocean-Atmosphere Interaction
      • Ocean Time-series
      • US Biogeochemical-Argo
  • Activities
    • 20 years of OCB Symposium – 18 November 2026
    • OCB Webinars
    • Summer Workshop
    • Guidelines for OCB Workshops & Activities
    • Topical Workshops
      • 7th DMS(P) Symposium
      • Marine Virus Workshop
      • Completed
        • CMIP6 Models Workshop
        • Coastal BGS Obs with Fisheries
        • C-saw extreme events workshop
        • Expansion of BGC-Argo and Profiling Floats
        • Fish, fisheries and carbon
        • Future BioGeoSCAPES program
        • GO-BCG Scoping Workshop
        • Lateral Carbon Flux in Tidal Wetlands
        • Leaky Deltas Workshop
        • Marine CDR Workshop
        • Ocean Nucleic Acids ‘Omics
        • Pathways Connecting Climate Changes to the Deep Ocean
    • Small Group Activities
      • BECS Benthic Ecosystem and Carbon Synthesis WG
      • Metabarcoding intercal WG
      • Meta-eukomics WG
      • Metaproteomic Intercomparison
      • SedMIP
      • Recently completed
        • Aquatic Continuum OCB-NACP Focus Group
        • Arctic-COLORS Data Synthesis
        • Carbon Isotopes in the Ocean Workshop
        • CMIP6 WG
        • Filling the gaps air–sea carbon fluxes WG
        • Fish Carbon WG
        • mCDR
        • Mixotrophs & Mixotrophy WG
        • N-Fixation WG
        • Ocean Carbonate System Intercomparison Forum
        • Ocean Carbon Uptake WG
        • OOI BGC sensor WG
        • Operational Phytoplankton Observations WG
        • Phytoplankton Taxonomy WG
    • Other Workshops
    • Science Planning
      • Coastal CARbon Synthesis (CCARS)
      • North Atlantic-Arctic
    • Ocean Acidification PI Meetings
    • Training Activities
      • PACE Hackweek 2025
      • PACE Hackweek 2024
      • PACE Training Activity 2022
  • Science Support
    • OCB Activity Proposal Solicitation
    • Guidelines for OCB Workshops & Activities
    • Data management and archival
    • Early Career
    • Funding Sources
    • Jobs & Postdocs
    • Meeting List
    • OCB Topical Websites
      • Ocean Fertilization
      • Trace gases
      • US IIOE-2
    • Outreach & Education
    • Promoting your science
    • Student Opportunities
    • Travel Support
  • Publications
    • OCB Workshop Reports
    • Science Planning and Policy
    • Newsletter Archive
  • Science Highlights
  • News

Archive for biological pump – Page 7

Nutrient Distributions Reveal the Fate of Sinking Particles

Posted by mmaheigan 
· Monday, November 21st, 2016 

The ocean’s “biological pump” regulates the atmosphere-ocean partitioning of carbon dioxide (CO2), and has likely contributed to significant climatic changes over Earth’s history (1, 2). It comprises two processes, separated vertically in the water column: (i) production of organic carbon and export from the surface euphotic zone (0-100m), mostly as sinking particles; and (ii) microbial remineralization of organic carbon to CO2 in deeper waters, where it cannot exchange with the atmosphere.

The depth of particulate organic carbon (POC) remineralization controls the longevity of carbon storage in the ocean (3), and strongly influences the atmospheric CO2 concentration (4). CO2 released in the mesopelagic zone (100-1000m) is returned to the atmosphere on annual to decadal timescales, whereas POC remineralization in the deep ocean (>1000m) sequesters carbon for centuries or longer (5). A common metric for the efficiency of the biological pump is thus the fraction of sinking POC that reaches the deep ocean before remineralization (6), referred to as the particle transfer efficiency, or Teff.

Currently, the factors that govern particle remineralization depth are poorly understood and crudely represented in climate models, compared to the lavish treatment of POC production by autotrophic communities in the surface (7). This compromises our ability to predict the biological pump’s response to anthropogenic warming, and its potential feedback on atmospheric CO2 (8). Over the last decade, a number of studies have identified a promising path towards closing this gap. If systematic spatial variations inTeff can be identified throughout the modern ocean, we might discern their underlying environmental or ecological causes (9, 10). However, direct observations from sediment traps are too sparse to constrain time-mean particle fluxes through the mesopelagic zone at the global scale, and no consensus pattern of Teff has emerged from these analyses.
Particle flux reconstruction

Instead of relying on sparse particle flux observations, a recent study took an alternative approach, leveraging the geochemical signatures that are left behind when particles remineralize (11). Products of remineralization include inorganic nutrients like phosphate (PO43-), whose global distributions are well characterized by hundreds of thousands of shipboard observations (12). In shallow subsurface waters, nutrient accumulation reflects the remineralization of both organic particles and dissolved organic matter, which is advected and entrained from the euphotic zone. Dissolved organic phosphorous (DOP) decomposes rapidly, and is almost completely absent

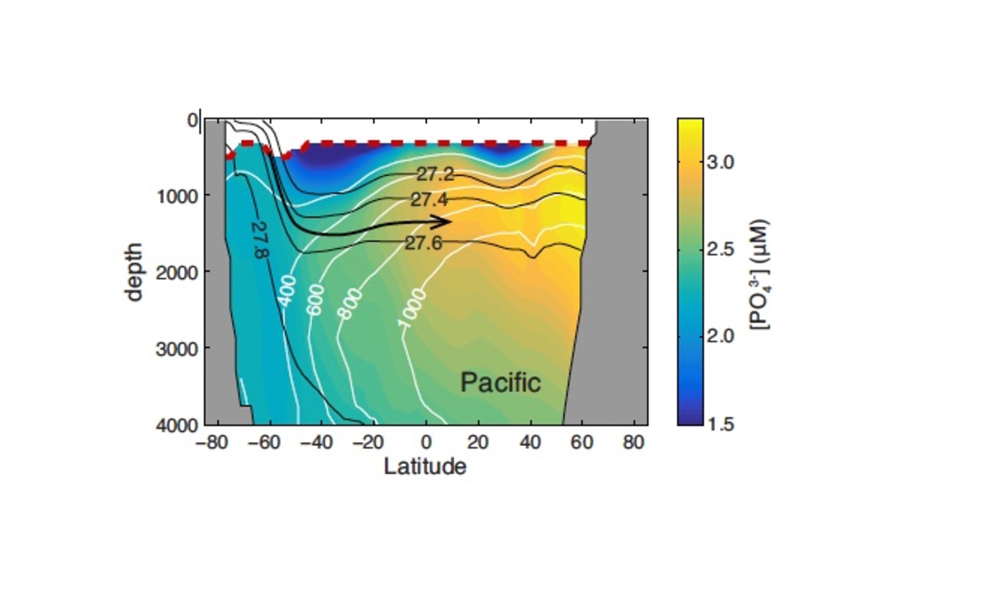
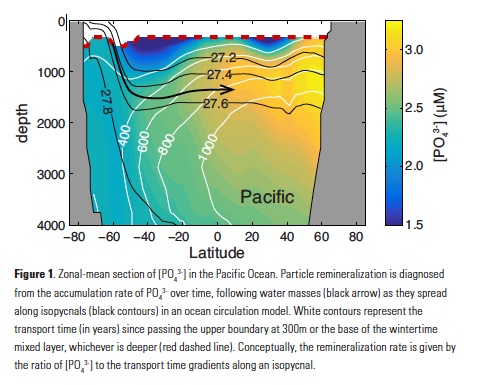
In shallow subsurface waters, nutrient accumulation reflects the remineralization of both organic particles and dissolved organic matter, which is advected and entrained from the euphotic zone. Dissolved organic phosphorous (DOP) decomposes rapidly, and is almost completely absent by depths of ~300m in the stratified low latitude ocean (13), and below the wintertime mixed layer in high latitudes (14). Deeper in the water column, particulate organic phosphorous (POP) remineralization is the only process that generates PO43- within water masses as they flow along isopycnal surfaces (Fig. 1). Rates of POP remineralization can therefore be diagnosed from the accumulation rate of PO43- along transport pathways in an ocean circulation model. This calculation requires a very faithful representation of the large-scale circulation, as provided by the Ocean Circulation Inverse Model (OCIM), whose flow fields are optimized to match observed water mass tracer distributions (15).

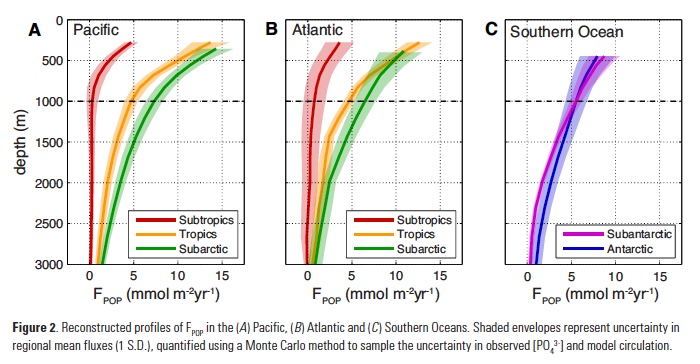
Assuming that organic matter burial in sediments is negligible, the integrated POP remineralization beneath a given depth horizon is equal to the flux of POP (FPOP) through that horizon, allowing complete reconstruction of flux profiles from ~300m to the deep ocean. Averaging these fluxes over large ocean regions serves to extract the large-scale signal from small-scale noise (Fig. 2). Regional-mean FPOP profiles show striking differences in shape and magnitude between subarctic, tropical, and subtropical regions, which are remarkably consistent between the Pacific and Atlantic Oceans (Fig 2a,b). FPOP near 300m is similar in subarctic and tropical zones, but attenuates faster through the mesopelagic in the tropics, reaching values of ~5mmol m-2yr-1 at 1000m, compared to ~7mmol m-2yr-1 in subarctic oceans. Subtropical FPOP attenuates even faster, and is indistinguishable from zero throughout most of the water column. In the Southern Ocean, FPOP is ~5mmol m-2yr-1 at 1000m in both the Antarctic and subantarctic regions, but the subantarctic flux profile attenuates slightly faster (Fig. 2c).
Patterns of transfer efficiency and underlying mechanisms

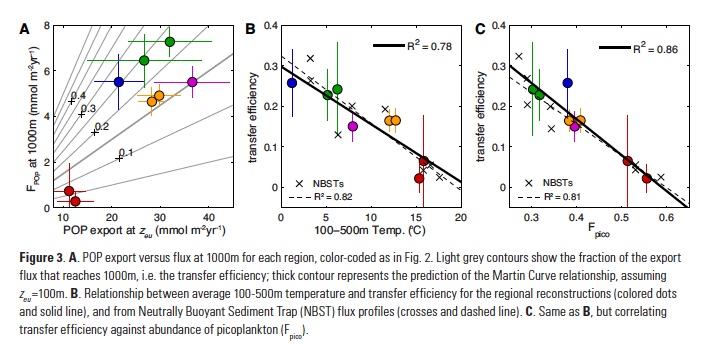
While these reconstructions place a robust constraint on POP fluxes to the deep ocean, they do not constrain rates of POP export at the base of the euphotic zone (zeu) that are needed to estimate the particle transfer efficiency (Teff). Remote sensing approaches are widely used to estimate large-scale organic carbon export, which can be converted to POP using an empirical relationship for particulate P:C ratios (16). However, multiple algorithms have been proposed to estimate net primary production and convert it to export, yielding widely different regional-mean rates (11). One way to pare down this variability is to weight each algorithm based on its ability to reproduce tracer-based export estimates in each ocean region (17, 18). This yields an “ensemble” estimate for the areal-mean POP export rate in each region, and an uncertainty range that reflects both observational error and the variability between satellite algorithms (Fig. 3a).

Combining the ensemble estimates of POP export with reconstructed FPOP at 1000m reveals a systematic pattern of transfer efficiency from zeu to the deep ocean (Fig. 3a).  The subtropics exhibit the lowest Teff of ~5%, significantly lower than expected from the canonical Martin Curve relationship (19), which is often considered to represent an “average” particle flux profile. In the tropics and the subantarctic zone of the Southern Ocean, Teff clusters close to the Martin Curve prediction of ~15%. The subarctic and Antarctic regions (i.e. high latitudes) are the most efficient at delivering the surface export flux to depth with Teff>25%, although these values are also associated with the largest uncertainty (Fig. 3a).

What controls the strong latitudinal variation of transfer efficiency? Particle flux attenuation is determined by the sinking speed and bacterial decomposition rate of particles: fast sinking and slow decomposition both result in greater delivery of organic matter to the deep ocean. Decomposition rates increase as a function of temperature in laboratory incubation studies (20), controlled by the temperature-dependence of bacterial metabolism. In a recent compilation of Neutrally Buoyant Sediment Trap (NBST) observations, particle flux attenuation was strongly correlated with upper ocean temperature between 100-500m (21), consistent with this effect. An almost identical temperature relationship explains ~80% of the variance in reconstructed regional Teff estimates (Fig. 3b).

An equally compelling argument can be made for particle sinking speeds controlling the pattern of Teff. According to the current paradigm of marine food webs (22), communities dominated by small phytoplankton export small particles that sink slowly, relative to the large aggregates and fecal pellets produced when large plankton dominate. The fraction of photosynthetic biomass contributed by tiny picoplankton (Fpico) varies from <30% in subarctic regions to >55% in oligotrophic subtropical regions (23), and explains ~86% of the variance in reconstructed Teff (Fig. 3c). Fpico also predicts flux attenuation in NBST profiles as skillfully as upper-ocean temperature (R2 = 0.81 and 0.82 respectively), but was not considered previously (21). Due to the spatial covariation of these factors in the ocean, statistical analysis alone is insufficient to determine the relative contributions of temperature and particle size to latitudinal variations in transfer efficiency.
Conclusions and future directions

Reconstructing deep-ocean particle fluxes has left us with a clearer understanding of the biological pump in the contemporary ocean and its climate sensitivity. Deep remineralization in high latitude regions results in efficient long-term carbon storage, whereas carbon exported in subtropical regions is recirculated to the atmosphere on short timescales (11). Atmospheric CO2 is likely more sensitive to increased high latitude nutrient utilization during glacial periods than previously recognized, whereas the expansion of subtropical gyres in a warming climate might result in a less efficient biological pump.

One caveat is that the new results highlighted here constrain POP transfer efficiency, not POC, and the two might be decoupled by preferential decomposition of one element relative to the other. The close agreement of these results with Neutrally Buoyant Sediment Trap observations (which measure POC) is encouraging, and suggests that the reconstructed pattern ofTeff is applicable to carbon. More widespread deployment of NBSTs, which circumvent the sampling biases of older sediment trap systems (24), would help confirm or refute this conclusion. A second limitation is that the wide degree of uncertainty in high latitude export rates (Fig. 3a) obscures estimates ofTeff in these regions. New tracer-based methods to integrate export across the seasonal cycle (25) will hopefully close this gap and enable more careful groundtruthing of satellite predictions.

Two plausible mechanisms –particle size and temperature – have been identified to explain large latitudinal variations in transfer efficiency, and new observational systems hold the potential to disentangle their effects. Underwater Visual Profilers (UVP) can now accurately resolve the size distribution of particles in mesopelagic waters (26). Although UVPs provide only instantaneous snapshots (quite literally) of the particle spectrum rather than time-mean properties, large compilations of these data will help establish the spatial pattern of particle size and its relationship to microbial community structure. In parallel, ongoing development of the RESPIRE particle incubator will allow for in-situ measurement of POC respiration (27), and better establish its temperature sensitivity.

Over the next few years, the upcoming EXport Processes in the Ocean from RemoTe Sensing (EXPORTS) campaign stands to revolutionize our understanding of the fate of organic carbon (28). These insights will allow for a more balanced treatment of the “dark side” of the biological pump in global climate models, compared to euphotic zone processes, improving our predictions of biological carbon sequestration in a warming ocean.

Author

By Thomas Weber (University of Rochester)

Acknowledgment

This work was supported by NSF grant OCE-1635414 and the Gordon and Betty Moore Foundation (GBMF 3775).

References

1. J. L. Sarmiento et al., Philos. Trans. R. Soc. A Math. Phys. Eng. Sci. 325, 3–21 (1988).
2. A. Mart.nez-Garc.a et al., Science 343, 1347–50 (2014).
3. U. Passow, C. Carlson, Mar. Ecol. Prog. Ser. 470, 249–271 (2012).
4. E. Y. Kwon, F. Primeau, J. L. Sarmiento, Nat. Geosci. 2, 630–635 (2009).
5. T. Devries, F. Primeau, C. Deutsch, Geophys. Res. Lett. 39, 1–5 (2012).
6. P. J. Lam, S. C. Doney, J. K. B. Bishop, Glob. Biogeochem. Cycles. 25, 1–14 (2011).
7. J. K. Moore, S. C. Doney, J. a. Kleypas, D. M. Glover, I. Y. Fung, Deep. Res. Part II Top. Stud. Oceanogr. 49, 403–462 (2002).
8. L. Bopp et al., Biogeosci. 10, 6225–6245 (2013).
9. S. a. Henson, R. Sanders, E. Madsen, Glob. Biogeochem. Cycles. 26, 1–14 (2012).
10. M. J. Lutz, K. Caldeira, R. B. Dunbar, M. J. Behrenfeld, J. Geophys. Res. 112, C10011 (2007).
11. T. Weber, J. A. Cram, S. W. Leung, T. Devries, C. Deutsch, Proc. Nat. Acad. Sci. 113, 8606–8611 (2016).
12. H. E. Garcia et al., NOAA World Ocean Atlas (2010).
13. J. Abell, S. Emerson, P. Renaud, J. Mar. Res. 58, 203–222 (2000).
14. S. Torres-Vald.s et al., Glob. Biogeochem. Cycles. 23, 1–16 (2009).
15. T. Devries, Glob. Biogeochem. Cycles. 28, 631–647 (2014).
16. E. D. Galbraith, A. C. Martiny, Proc. Nat. Acad. Sci., 201423917 (2015).
17. M. K. Reuer, B. A. Barnett, M. L. Bender, P. G. Falkowski, M. B. Hendricks, Deep. Res. Part I Oceanogr. Res. Pap. 54, 951–974 (2007).
18. S. Emerson, Glob. Biogeochem. Cycles. 28, 14–28 (2014).
19. J. H. Martin, G. A. Knauer, D. M. Karl, W. W. Broenkow, Deep Sea Res. Part A, Oceanogr. Res. Pap. 34, 267–285 (1987).
20. M. H. Iversen, H. Ploug, Biogeosciences. 10, 4073–4085 (2013).
21. C. M. Marsay, R. J. Sanders, S. A. Henson, K. Pabortsava, E. P. Achterberg, Proc. Nat. Acad. Sci., 112, 1089–1094 (2014).
22. D. A. Siegel et al., Glob. Biogeochem. Cycles. 28, 181–196 (2014).
23. T. Hirata et al., Biogeosci. 8, 311–327 (2011).
24. K. O. Buesseler et al., Science 316, 567–570 (2007).
25. S. M. Bushinsky, S. Emerson, Glob. Biogeochem. Cycles. 29, 2050–2060 (2015).
26. M. Picheral et al., Limnol. Oceanogr. Methods. 8, 462–473 (2010).
27. A. M. P. McDonnell, P. W. Boyd, K. O. Buesseler, Glob. Biogeochem. Cycles. 29, 175–193 (2015).
28. D. A. Siegel et al., Front. Mar. Sci. 3, 1–10 (2016).
Marine mixotrophs exploit multiple resource pools to balance supply and demand

Posted by mmaheigan 
· Sunday, November 20th, 2016 

“So, in the sea, there are certain objects concerning which one would be at a loss to determine whether they be animal or vegetable.”  Aristotle, The History of Animals

Our understanding of marine ecosystems is strongly influenced by the terrestrial macroscopic world we see around us. For example, the distinction between phytoplankton and zooplankton reflects the very familiar divide between plants and animals. Mixotrophs are organisms that blur this distinction by combining photosynthetic carbon fixation and the uptake of inorganic nutrients with the ingestion of living prey (1). In the macroscopic terrestrial realm, the obvious examples of mixotrophs are the carnivorous plants. These organisms are so well known because they confound the otherwise clear divide between autotrophic plants and heterotrophic animals – in terrestrial environments, mixotrophs are the exception rather than the rule. There appear to be numerous reasons for this dichotomy involving constraints on surface area to volume ratios, the energetic demands of predation, and access to essential nutrients and water. Without dwelling on these aspects of macroscopic terrestrial ecology, it appears that many of the most important constraints are relaxed in aquatic microbial communities. Plankton have no need for the fixed root structures that would prevent motility, and in the three-dimensional fluid environment, they are readily exposed to both inorganic nutrients and prey. In addition, their small size and high surface area to volume ratios increase the potential efficiency of light capture and nutrient uptake. As such, mixotrophy is a common and widely recognised phenomenon in marine ecosystems. It has been identified in a very broad range of planktonic taxa and is found throughout the eukaryotic tree of life. Despite its known prevalence, the potential impacts of mixotrophy on the global cycling of nutrients and carbon are far from clear. In this article, I discuss the ecological niche and biogeochemical role of mixotrophs in marine microbial communities, describing some recent advances and identifying future challenges.

A ubiquitous and important strategy

Mixotrophy appears to be a very broadly distributed trait, appearing in all marine biomes from the shelf seas (2) to the oligotrophic gyres (3), and from the tropics (4) to the polar oceans (5). Within these environments, mixotrophy is often a highly successful strategy. For example, in the subtropical Atlantic, mixotrophic plankton make up >80% of the pigmented biomass, and are also responsible for 40-95% of grazing on bacteria (3, 4). Similar abundances and impacts have also been observed in coastal regions (2, 6).

How does the observed prevalence of mixotrophy affect the biogeochemical and ecological function of marine communities? To understand the potential answers to this question, it is helpful to review the constraints associated with the assumption of a strict dichotomy between autotrophic phytoplankton and heterotrophic zooplankton. Within this paradigm, primary production is restricted to the base of the food web, tightly coupled to the supply of limiting nutrients. Furthermore, the vertical export of
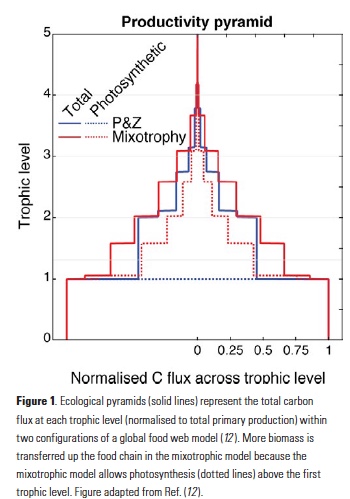
carbon is limited by the supply of exogenous (or “new”) nutrients (7), since any local regeneration of nutrients from organic matter is also associated with the local remineralisation of dissolved inorganic carbon. Energy and biomass are passed up the food web, but the transfer across trophic levels is highly inefficient (8) (Fig. 1) because the energetic demands of strictly heterotrophic consumers can only be met by catabolic respiration.

In the mixotrophic paradigm, several of these constraints are relaxed. Primary production is no longer exclusively dependent on the supply of inorganic nutrients because mixotrophs can support photosynthesis with nutrients derived from their prey. This mechanism takes advantage of the size-structured nature of marine communities (9), with larger organisms avoiding competitive exclusion by eating their smaller and more efficient competitors (10-12). In addition, the energetic demands of mixotrophic consumers can be offset by phototrophy, leading to increased efficiency of carbon transfer through the food web (Fig. 1). These two mechanisms dictate that mixotrophic ecosystems can fix and export more carbon for the same supply of limiting nutrient, relative to an ecosystem strictly divided between autotrophic phytoplankton and heterotrophic zooplankton (12).

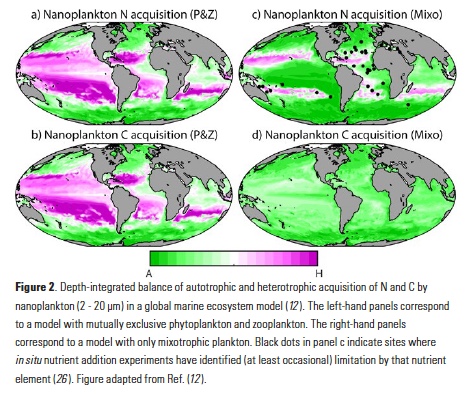
The trophic flexibility associated with mixotrophy appears likely to have a profound effect on marine ecosystem function at the global scale. Fig. 2 contrasts the simulated fluxes of carbon and nitrogen through the intermediate nanoplankton (2-20 μm diameter) size class of a global ecosystem model (12). The left-hand maps show the balance of autotrophic and heterotrophic resource acquisition in a model with mutually exclusive phytoplankton and zooplankton. At low latitudes and especially in the
oligotrophic subtropical gyres, the inorganic nitrogen supply is acquired almost exclusively by the smallest and most competitive phytoplankton (not shown). This leaves an inadequate supply for larger and less competitive phytoplankton, and as such, the larger size classes are dominated by zooplankton (as indicated by the purple shading in Fig. 2a, b). In the more productive polar oceans and upwelling zones, grazing pressure prevents the smaller phytoplankton from exhausting the inorganic nitrogen supply, leaving enough for the larger phytoplankton to thrive in these regions (as indicated by the green shading).

The right-hand maps in Fig. 2 show the balance of autotrophic and heterotrophic resource acquisition in the intermediate size-class of an otherwise identical model containing only mixotrophic plankton. As in the model with mutually exclusive phytoplankton and zooplankton, the inorganic nitrogen supply in the oligotrophic gyres is exhausted by the smallest phytoplankton (see the purple shading in Fig. 2c). However, Fig. 2d indicates that this is not enough to stop photosynthetic carbon fixation among the mixotrophic nanoplankton. The nitrogen acquired from prey is enough to support considerable photosynthesis in a size class for which phototrophy would otherwise be impossible. For the same supply of inorganic nutrients, this additional supply of organic carbon serves to enhance the transfer of energy and biomass through the microbial food web, increasing community carbon:nutrient ratios and leading to as much as a three-fold increase in mean organism size and a 35% increase in vertical carbon flux (12).

Trophic diversity and ecosystem function

Marine mixotrophs are broadly distributed across the eukaryotic tree of life (13). The ability to combine photosynthesis with the digestion of prey has been identified in ciliates, cryptophytes, dinoflagellates, foraminifera, radiolarians, and coccolithophores (14). Perhaps the only major group with no identified examples of mixotrophy are the diatoms, which have silica cell walls that may hinder ingestion of prey. While some mixotroph species are conceptually more like plants (that eat), others are more like animals (that photosynthesise). A number of conceptual models have been developed to account for this observed diversity. One scheme (15) identified three primarily autotrophic groups that use prey for carbon, nitrogen or trace compounds, and two primarily heterotrophic groups that use photosynthesis to delay starvation or to increase metabolic efficiency. More recently, an alternative classification (16, 17) identified three key groups on a spectrum between strict phototrophy and strict phagotrophy. According to this classification, primarily autotrophic mixotrophs can synthesise and fully regulate their own chloroplasts, whereas more heterotrophic forms must rely on chloroplasts stolen from their prey. Among this latter group, the more specialised species exploit only a limited number of prey species, but can manage and retain stolen chloroplasts for relatively long periods. In contrast, generalist mixotrophs target a much wider range of prey, but any stolen chloroplasts will degrade within a matter of hours or days (18).

This diversity of trophic strategies is clearly more than most biogeochemical modellers would be prepared to incorporate into their global models. Nonetheless, many of the conceptual groups identified above are associated with the ability of mixotrophs to rectify the often-imbalanced supply of essential resources in marine ecosystems (19). This is clearly relevant to the coupling of elemental cycles in the ocean, and it appears likely that the relative abundance of different trophic strategies can impact the biogeochemical function of marine communities (1, 20). For example, recent work suggests that a differential temperature sensitivity of autotrophic and heterotrophic processes can push mixotrophic species towards a more heterotrophic metabolism with increasing temperatures (21). An important goal is therefore to accurately quantify and account for the global-scale effects of mixotrophy on the transfer of energy and biomass through the marine food web and the export of carbon into the deep ocean. We also need to assess how these effects might be sensitive to changing environmental conditions in the past, present, and future.

These processes are not resolved in most contemporary models of the marine ecosystem, which are often based on the representation of a limited number of discrete plankton functional types (22). In terms of resolving mixotrophy, it is not the case that these models have overlooked the one mixotrophic group. Instead, it may be more accurate to say that the groups already included have been falsely divided between two artificially distinct categories. As such, modelling mixotrophy in marine ecosystems is not just a case of increasing complexity by adding an additional mixotrophic component. Instead, progress can be made by understanding the position, connectivity, and influence of mixotrophic and non-mixotrophic organisms within the food web as an emergent property of their environment, ecology, and known eco-physiological traits. This is not a simple task, but progress might be made by identifying the fundamental traits that underpin the observed diversity of functional groups. To this end, a recurring theme in mixotroph ecology is that plankton exist on a spectrum between strict autotrophy and strict heterotrophy (14, 23, 24). Competition along this spectrum is typically framed in terms of the costs and benefits of different modes of nutrition. Accurate quantification of these costs and benefits should allow for a much clearer understanding of the trade-offs between different mixotrophic strategies (25), and how they are selected in different environments. In the future, a combination of culture experiments, targeted field studies, and mathematical models should help to achieve this goal, such that this important ecological mechanism can be reliably and parsimoniously incorporated into global models of marine ecosystem function.

Author

Ben Ward (University of Bristol)

References

1. Stoecker, D. K., Hansen, P. J., Caron, D. A. & Mitra, Annual Rev. Marine Sci. 9, forthcoming (2017).
2. Unrein, F., Gasol, J. M., Not, F., Forn, I. & Massana, R. The ISME Journal 8, 164–176 (2013).
3. Zubkov, M. V. & Tarran, G. A. Nature 455, 224–227 (2008).
4. Hartmann, M. et al. Proc. Nat. Acad. Sci. 5756–5760 (2012). doi:10.1073/pnas.1118179109
5. Gast, R. J. et al. J. Phycol. 42, 233–242 (2006).
6. Havskum, H. & Riemann, B. Marine Ecol. Prog. Ser. 137, 251–263 (1996).
7. Dugdale, R. C. & Goering, J. J. Limnol. Oceanogr. 12, 196–206 (1967).
8. Lindeman, R. L. Ecol. 23, 399–417 (1942).
9. Sieburth, J. M., Smetacek, V. & Lenz, J. Limnol. Oceanogr. 23, 1256–1263 (1978).
10. hingstad, T. F., Havskum, H., Garde, K. & Riemann, B. Ecol. 77, 2108–2118 (1996).
11. Våge, S., Castellani, M., Giske, J. & Thingstad, T. F. Aquatic Ecol. 47, 329–347 (2013).
12. Ward, B. A. & Follows, M. J. Proc. Nat. Acad. Sci. 113, 2958–2963 (2016).

Marine particles: Distribution, composition, and role in scavenging of TEIs

Posted by mmaheigan 
· Sunday, July 3rd, 2016 

GEOTRACES and particles in the ocean

GEOTRACES is an international program to study the global marine biogeochemical cycles of trace elements and their isotopes (TEIs). The program’s guiding mission is to “identify processes and quantify fluxes that control the distributions of key TEIs in the ocean” (1).

Particles represent a key parameter for the GEOTRACES program because of their role as sources, sinks, and in the internal cycling of so many TEIs (1, 2). Particles in the ocean fall into two classes: 1. Those that have sources external to the system such as lithogenic material carried by atmospheric transport, river, or lateral transport from continental margin sediments; and 2. those that are produced internally in the system, primarily by biological production, but also by authigenic mineral precipitation (2).

External particle sources such as mineral dust deposition and sediment resuspension act as sources of dissolved TEIs when they partially dissolve in seawater. Conversely, dissolved TEIs are removed by active biological uptake or passive adsorption onto particles surfaces, followed by particle removal by aggregation and sinking. Indeed, the biological and abiotic interactions of dissolved TEIs with particles determine the residence time of a dissolved TEI.

In most open ocean basins away from ocean floor boundaries, external sources of particles are dwarfed by the much greater biological production and destruction of particles. Particle cycling in most open ocean basins is thus dominated by the biological pump, the processes by which suspended particles are produced by photosynthesis in the euphotic zone at the surface, and are then abiotically or biologically aggregated into larger particles that can sink into the abyss (3).

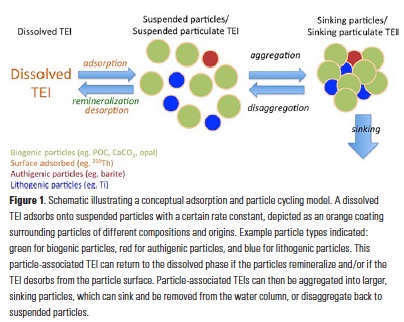
As particulate organic carbon (POC) cycles through processes such as aggregation, disaggregation, remineralization, and sinking (collectively referred to here as particle dynamics), other particle phases are swept along for the ride, including other major components such as biologically precipitated minerals (especially CaCO3 and opal), as well as lithogenic and authigenic particles, and scavenged TEIs adsorbed to the surfaces of other particles (Fig. 1).

In this article, I will briefly review the role of particle composition on the scavenging of TEIs.

Scavenging: A two-step removal process

Most adsorption of TEIs likely occurs onto small, suspended particles, which are usually more abundant, have more available surface area, and have a longer residence time in the water column than large, sinking particles. For TEIs to be removed from the water column, the suspended particles must then be aggregated into larger, sinking particles. There are thus two distinct steps for the removal of a dissolved TEI by scavenging: 1) adsorption onto suspended particle surfaces, followed by 2) removal via the aggregation of suspended particles onto larger particles that sink out of the water column. Fig. 1 shows a very simple schematic illustrating these basic processes. The adsorption step is governed by the affinity of a TEI for a particular particle surface, and the removal step is governed by the particle dynamics that package suspended particles into large, sinking aggregates, and are the focus of studies of the biological pump. The removal of TEIs by scavenging thus intimately links one of OCB’s scientific goals, the understanding of the biological carbon pump, to GEOTRACES’s mission to identify processes and quantify fluxes that control the distributions of key TEIs in the ocean.

Particle concentration and composition: horizontal and vertical variations

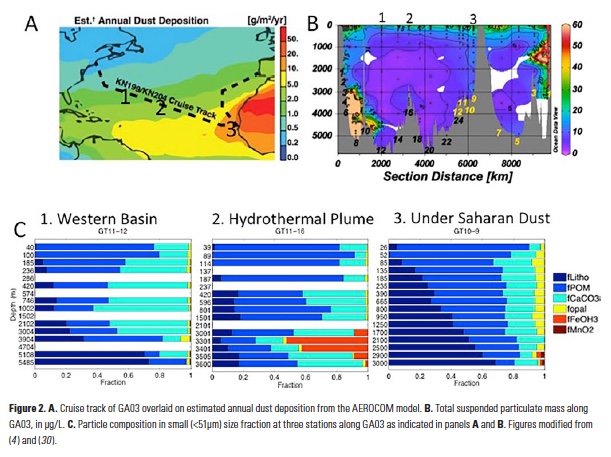
Particles collected in the ocean are a heterogeneous mixture of biogenic, lithogenic, and authigenic (precipitated in-situ) components. The relative proportions of these different components vary geographically and with depth. Fig. 2 shows the distribution of total particle concentration from GA03, the U.S. GEOTRACES North Atlantic Zonal Transect cruise in 2010/2011, as well as the changing composition of small (<51 mm) particles at three stations along the transect (4). Particle concentrations are highest at the surface and at the margins, where biological production is highest. It is clear that particulate organic matter (POM) dominates particle composition in the upper 100 m, making up more than 70% of the suspended particle mass at all three stations. The balance in the upper 100 m is mostly made of other biogenic components such as CaCO3 and opal, with a small contribution from lithogenic particles directly under the Saharan dust  plume. At all stations, the inorganic components (everything except for POM) become relatively more important with depth as POM is remineralized. In the eastern half of the basin, lithogenic particles make up the largest fraction of particle mass, accounting for >50% of particle mass below 1500 m. In the western half of the basin, further from the Saharan dust source, lithogenic particles are not as important, and CaCO3 makes up the largest fraction (~50%) of particle mass between 500 – 3000 m. A special case is found in a station over the Mid-Atlantic Ridge, where iron oxyhydroxides from the hydrothermal plume make up ~50% of the particle mass. Iron and manganese oxyhydroxides are rarely dominant components of particle mass, except in special situations such as hydrothermal plumes, but may exert a particularly large influence on TEI adsorption (5, 6 ).

Studies suggest that particle composition may affect both the affinity of dissolved TEIs for adsorbing onto particle surfaces (2), and the vertical flux of particles from the water column (7-9). Horizontal and vertical changes in particle composition thus allow us to test hypotheses of the importance of particle composition on both steps in the scavenging of TEIs.

Effect of particle composition on adsorption of TEIs

The affinity of TEIs to particles has typically been characterized by a partition coefficient, Kd, which is calculated empirically as:

Prior to the GEOTRACES program, the effect of particle composition on TEI adsorption affinity had been studied in the field using sediments and sinking particles collected in sediment traps. The affinity of trace metals to marine sediments of different compositions varied: Some trace metals (Cs, Be, Sn, and Fe) had a higher affinity to sediments dominated by aluminosilicate clay minerals, and others (Ba, Cd, Zn, Mn, and Co) had a higher affinity to sediments enriched in Mn oxyhydroxides (10). In the water column, correlations between the partition coefficient of 230Th and particle composition in sediment trap particles from around the world have variously implied that the scavenging efficiency of 230Th is controlled by CaCO3 (11, 12), lithogenic material (13, 14), and/or Mn oxyhydroxides (15). Studies that span strong opal gradients across the Polar Front in the Southern Ocean show higher partition coefficients for 231Pa scavenging in areas of high opal content (11, 16). 231Pa is generally not as particle-reactive as 230Th in the open ocean, but is often removed with equal efficiency as 230Th in near-margin areas (e.g., 17), presumably because opal is more important in margin settings. The Arctic, on the other hand, displays the opposite 230Th/231Pa removal signal, with 231Pa removal less efficient relative to 230Th at the margins compared to the open ocean (18).

Since TEIs adsorb primarily onto suspended particles rather than sinking particles, studying the correlations between partition coefficients and suspended particles may resolve some of the discrepancies observed in the sediment trap studies (c.f., 2).

The GEOTRACES GA03 North Atlantic Zonal Transect has provided the first opportunity to investigate the correlation between partition coefficients of various TEIs and the particle composition of suspended particles in the ocean. Thus far, this has been done for 230Th and 231Pa partition coefficients, with Mn and Fe oxyhydroxides emerging as key controlling phases and opal having no controlling effect (5). The North Atlantic is very opal-poor (Fig. 2), so particles collected from more diatom-rich regions are needed to examine the potential of opal as a controlling phase. Other studies are underway to study the  particle affinities of Hg (19), Po (20), and Pb (6) on this same North Atlantic transect. Subsequent U.S. GEOTRACES sections (GP16—Eastern Tropical South Pacific Zonal Transect and GN01—Western Arctic) will also have full ocean depth size-fractionated particle concentration and composition, allowing us to examine samples from different biogeochemical provinces, and hopefully expanding the range of particle compositions.

TEIs as tracers of scavenging rates and particle dynamics

The unprecedented data sets from GEOTRACES are also allowing us to estimate adsorption and desorption rate constants (Fig. 1) from inverse modeling of the observations of dissolved and particulate TEIs and particle concentrations (19, 21, 22). This gives us a kinetic view of the scavenging process to complement the empirically-derived partition coefficients, which are often viewed as representing equilibrium constants. Applying inverse modeling approaches to observations of the distributions of size-fractionated particles and particulate TEIs can also allow us to estimate rates of particle remineralization, aggregation, disaggregation, and sinking (21, 23). This approach requires only that a conceptual model relating the suspended and sinking particle size fractions be applied to observations of particle mass and particulate TEIs, and does not require knowledge about which specific physical or biological processes are responsible for particle transformations. For example, Fig. 1 illustrates a simple conceptual model in which a pool of suspended particles can be lost to the dissolved phase through remineralization, or by aggregation into sinking particles; conversely, sinking particles can sink, or can be disaggregated back into suspended particles. By assuming that particulate TEIs are simply part of the overall particle pool (e.g., a coating on organic particles in the case of radiogenic TEIs such as 230Th or as part of a lithogenic particle in the case of a TEI such as Ti) and thus are subject to the same rates of particle transformations as the major phases such as POC, we can apply the same conceptual model to observations of particle mass and to observations of particulate TEI to better constrain the rates of these transformations (23). As some of these rates such as aggregation and disaggregation are notoriously difficult to measure directly, these inverse approaches offer a way forward to quantify these important processes.

Particle composition and the biological pump

In addition to its effect on scavenging efficiency, particle composition has also been implicated as an important factor in the strength and efficiency of the biological pump. Several meta-analyses of global deep (>1000 m) sediment trap data showed strong correlations between POC flux and mineral flux (7-9), leading to the development of the “ballast hypothesis.” The mechanisms to explain the correlations, which are still being debated (24, 25), range from mineral protection of POC (8), mineral contribution to particle excess density (7), scavenging of mineral particles by POC (26), and minerals as proxies for particle packaging, POC lability, and ecosystem structure (9, 27-29).

Although the GA03 dataset is based on size-fractionated particle samples collected by in-situ filtration rather than sinking particles collected by sediment traps, we can nonetheless examine whether there is a correlation between POC and ballast minerals in small or large particle size fractions. We found that POC concentration in large (>51 mm) particles was not consistently correlated with any of the potential ballast minerals CaCO3, opal, and lithogenic particles (4).The lack of strong correlations within this regional dataset is consistent with the idea that ballast mineral correlations with POC may only emerge in global datasets that combine different biogeochemical provinces (25).

Outlook

The GEOTRACES program is not only rapidly expanding global observations of dissolved TEIs, but it is also the latest major program to systematically sample particle distributions since JGOFS and GEOSECS (2). These particle measurements are not only helping us understand the processes controlling TEI distributions, but the TEI measurements can also be used as tracers for quantifying key processes of particle cycling. Both GEOTRACES and OCB can benefit from the insights gained in each program.

Author

Phoebe J. Lam (Department of Ocean Sciences, University of California, Santa Cruz)

References

1. GEOTRACES, Scientific Committee on Oceanic Research, Ed. (Baltimore, Maryland, 2006).
2. C. Jeandel et al., Progress in Oceanography 133, 6 (4//, 2015).
3. C. L. De La Rocha, in Treatise on Geochemistry, H. Elderfield, K. K. Turekian, Eds. (Elsevier, 2003), vol. 6: The Oceans and Marine Geochemistry, pp. 83-111.
4. P. J. Lam et al., Deep Sea Research Part II: Topical Studies in Oceanography 116, 303 (6//, 2015).
5. C. T. Hayes et al., Marine Chemistry 170, 49 (3/20/, 2015).
6. E. A. Boyle et al., paper presented at the 2016 Ocean Sciences Meeting, New Orleans, LA, USA, 2016.
7. C. Klaas, D. E. Archer, Global Biogeochemical Cycles 16, 1116 (Dec 5, 2002).
8. R. A. Armstrong et al., Deep-Sea Research Part II-Topical Studies in Oceanography 49, 219 (2002).
9. R. François et al., Global Biogeochemical Cycles 16, (Oct-Nov, 2002).
10 . L. S. Balistrieri, J. W. Murray, Geochimica Et Cosmochimica Acta 48, 921 (1984).
11. Z. Chase et al., Earth and Planetary Science Letters 204, 215 (Nov 30, 2002).
12. Z. Chase et al., Deep-Sea Research Part II-Topical Studies in Oceanography 50, 739 (2003).
13. S. D. Luo, T. L. Ku, Earth and Planetary Science Letters 220, 201 (Mar, 2004).
14. M. Roy-Barman et al., Earth and Planetary Science Letters 286, 526 (2009).
15. M. Roy-Barman et al., Earth and Planetary Science Letters 240, 681 (2005).
16. H. J. Walter et al., Earth and Planetary Science Letters 149, 85 (1997).
17. R. F. Anderson, M. P. Bacon, P. G. Brewer, Earth and Planetary Science Letters 66, 73 (1983).
18. H. N. Edmonds et al., Earth and Planetary Science Letters 227, 155 (Oct, 2004).
19. C. H. Lamborg et al., Philos T R Soc A, (accepted).
20. Y. Tang et al., paper presented at the 2016 Ocean Sciences Meeting, New Orleans, LA, USA, 2016.
21. O. Marchal, P. J. Lam, Geochimica Et Cosmochimica Acta 90, 126 (2012).
22. P. Lerner et al., Deep Sea Research Part I: Oceanographic Research Papers 113, 57 (7//, 2016).
23. P. J. Lam, O. Marchal, Annual Review of Marine Science 7, 159 (2015).

24. P. Boyd, T. Trull, Progress in Oceanography 72, 276 (2007).
25. J. D. Wilson, S. Barker et al., Global Biogeochemical Cycles 26, GB4011 (2012).
26. U. Passow, Geochemistry Geophysics Geosystems 5, (Apr 6, 2004).
27. P. J. Lam et al., Global Biogeochem. Cycles 25, GB3009 (2011).
28. S. A. Henson et al., Global Biogeochem. Cycles 26, GB1028 (2012).
29. S. Z. Rosengard et al., Biogeosciences 12, 3953 (2015).
30. D. C. Ohnemus, P. J. Lam, Deep Sea Research Part II: Topical Studies in Oceanography 116, 283 (6//, 2015).

« Previous Page

FilterbyKeyword

abundance acidification additionality advection africa aggregates air-sea air-sea interactions albedo algae alkalinity allometry amendments ammonium AMO AMOC anoxic Antarctic Antarctica anthro impacts anthropogenic carbon anthropogenic impacts appendicularia aquaculture aquatic continuum aragonite saturation arctic Argo argon arsenic artificial seawater assumptions AT Atlantic atmosphere atmospheric CO2 atmospheric nitrogen deposition authigenic carbonates autonomous platforms AUVs awb bacteria bathypelagic BATS BCG Argo benthic bgc argo bias bio-go-ship bio-optical bioavailability biogeochemical biogeochemical cycles biogeochemical models biogeochemistry Biological Essential Ocean Variables biological pump biomass biophysics bloom blue carbon bottom water boundary layer buffer capacity C14 CaCO3 calcification calcite carbon carbon-climate feedback carbon-sulfur coupling carbon 14 carbonate carbonate chemistry carbonate chemistry OAE carbonate system carbon budget carbon cycle carbon cycling carbon dioxide carbon export carbon fluxes carbon removal carbon sequestration carbon storage Caribbean CCA CCS CDOM changing marine chemistry changing marine ecosystems changing marine environments changing ocean chemistry chemical oceanographic data chemical speciation chemoautotroph chesapeake bay chl a chlorophyll circulation climate clouds CO2 CO3 coastal and estuarine coastal darkening coastal ocean cobalt Coccolithophores commercial community community composition competition conservation cooling effect copepod copepods coral reefs cruise CTD currents cyclone daily cycles data data access data assimilation database data management data product data sets Data standards DCM dead zone decadal trends decomposers decomposition deep convection deep ocean deep sea coral deep water deepwater horizon denitrification dense water deoxygenation depth diatoms DIC diel migration diffusion dimethylsulfide dinoflagellate dinoflagellates discrete measurements disequilibrium distribution DOC DOM domoic acid DOP dust DVM earth system ecological feedbacks ecology economics ecosystem management ecosystems eddy Education EEZ Ekman transport emissions ENSO enzyme equatorial current equatorial regions ESM estuarine and coastal carbon fluxes estuary euphotic zone eutrophication evolution export export fluxes export production extreme events faecal pellets fecal pellets feces feeding filter feeders filtration rates fire fish Fish carbon fisheries fishing fjord float floats fluid dynamics fluorescence food webs forage fish forams framework freshening freshwater frontal zone fronts functional role fungi future oceans gelatinous zooplankton gene transfer geochemistry geoengineering geologic time GEOTRACES glaciers gliders global carbon budget global oceam global ocean global ocean models global overturning circulation global warming go-ship gradient grazing greenhouse gas greenhouse gases Greenland ground truthing groundwater Gulf of Maine Gulf of Mexico Gulf Stream gyre harmful algal bloom heat waves high latitude human food human impact human well-being hurricane hydrogen hydrothermal hypoxia ice age iceberg ice cores ice cover industrial onset inland waters in situ inverse circulation ions iron iron fertilization iron limitation isotopes jellies katabatic winds kelvin waves krill kuroshio lab vs field lagoon land land-ocean continuum larvaceans lateral transport LGM lidar ligands light light attenuation lineage lipids low nutrient machine learning mangroves marine carbon cycle marine heatwave marine particles marine snow marine snowfall marshes mCDR mechanisms Mediterranean meltwater mesocosm mesopelagic mesoscale mesoscale processes metagenome metals methane methods microbes microbial processes microlayer microorganisms microplankton microplastics microscale microzooplankton midwater migration minerals mitigation mixed layer mixed layers mixing mixotrophs mixotrophy model modeling modeling atmosphere model validation mode water molecular diffusion MPT MRV multi-decade N2 n2o NAAMES NCP nearshore net community production net primary productivity new ocean state new technology Niskin bottle nitrate nitrogen nitrogen cycle nitrogen fixation nitrous oxide north atlantic north pacific North Sea NPP nuclear war nutricline nutrient budget nutrient cycles nutrient cycling nutrient limitation nutrients OA observations ocean-atmosphere ocean acidification ocean acidification data ocean alkalinity enhancement ocean carbon uptake & storage ocean carbon uptake and storage ocean color ocean interior ocean modeling ocean observatories ocean warming ODZ oil oligotrophic omics OMZ open ocean optics organic carbon organic particles oscillation outwelling overturning circulation oxidizing oxygen oxygen-deficient pacific paleoceanography PAR parameter optimization parasite particle flux particles partnerships pathway pCO2 PDO peat pelagic perturbation PETM pH phenology phosphate phosphorus photosynthesis physical processes physiology phytoplankton PIC piezophilic piezotolerant plankton POC polar polar regions policy pollutants precipitation predation predator-prey predators prediction pressure primary productivity Prochlorococcus productivity prokaryotes proteins pteropods pycnocline python radioisotopes rain redox remineralization remote sensing repeat hydrography residence time resource management respiration resuspension rivers rocky shore Rossby waves Ross Sea ROV salinity salt marsh satellite scale seafloor seagrass sea ice sea level rise seasonal seasonal effects seasonality seasonal patterns seasonal trends sea spray sea surface seawater collection seaweed secchi sediments sensor sensors sequestration shelf ocean shelf system shells ship-based obs ship-based observations shorelines siderophore silica silicate silicon cycle sink sinking sinking particles size SOCCOM soil carbon solubility pump southern ocean south pacific spatial covariations speciation spring mixing SST state estimation stoichiometry stratification subduction submesoscale subpolar subtropical sulfate surf surface surface ocean surface water surface waters Synechococcus technology teleconnections temperate temperature temporal covariations thermocline thermodynamics thermohaline thorium tidal time time-series time of emergence titration top predators total alkalinity trace elements trace metals trait-based transfer efficiency transient features trawling Tris trophic interactions trophic transfer tropical turbulence twilight zone upper ocean upper water column upwelling US CLIVAR uvp validation velocity gradient ventilation vertical flux vertical migration vertical transport viruses warming water clarity water column water mass water quality waves weathering western boundary currents wetlands winter mixing zooplankton

Copyright © 2026 - OCB Project Office, Woods Hole Oceanographic Institution, 266 Woods Hole Rd, MS #25, Woods Hole, MA 02543 USA Phone: 508-289-2838  •  Fax: 508-457-2193  •  Email: ocb_news@us-ocb.org

link to nsflink to noaalink to WHOI

Funding for the Ocean Carbon & Biogeochemistry Project Office is provided by the National Science Foundation (NSF) and the National Aeronautics and Space Administration (NASA). The OCB Project Office is housed at the Woods Hole Oceanographic Institution.